How does the Harris's hawk see?
The Harris's hawk (Parabuteo unicinctus) is a bird in the order Accipitriformes. Its eyes belong to the vision type Raptor telephoto: 4 cones (violet-sensitive), 2 foveas (deep central + temporal), the highest acuity measured, 35-50 deg binocular.
Measured in this species: sharpness, field of view, foveas, night vision and motion (flicker fusion). Measured core: measured values on at least 3 of the 6 dials. Every value below carries its evidence level and sources; nothing is typed by hand.
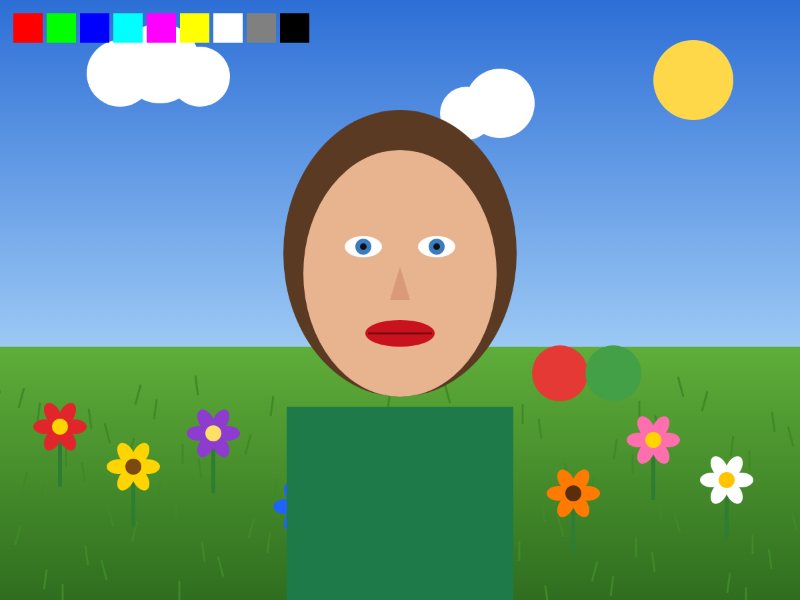
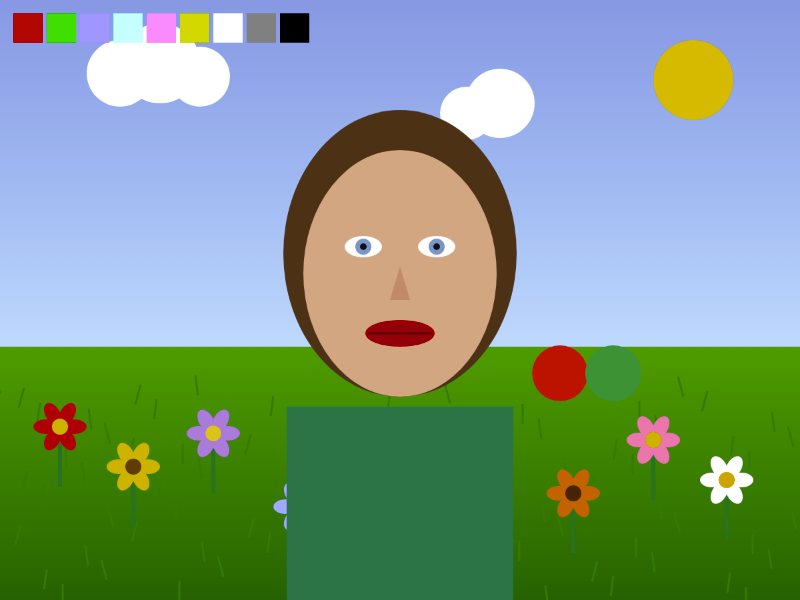
What stands out
- It has 4 colour receptor classes; people have 3.
- Its sharpest vision resolves 43.7 cycles per degree: the finest stripe pattern it can tell apart from grey.
- Its eyes cover about 277° around the head, with 47° seen by both eyes at once.
- It stops seeing flicker at 77.7 Hz, against 60 Hz for people in this dataset, so fast motion looks about 1.3 times slower to it.[12][13]
- Activity pattern: diurnal.
The six dials
Evidence levels: how the tiers work. "Measured" means a value measured in this species; "Estimated" values come from a close relative or an eye-size formula.
| Dial | Value | Evidence | Sources |
|---|---|---|---|
| Colour | Colour receptors 4 receptor classes: 405 nm (VS/SWS (violet)), 449 nm (SWS (blue)), 504 nm (MWS (green)), 567 nm (LWS (long)) receptor set of nearest measured relative Buteo buteo (same family Accipitridae) | Estimated | [1][2] |
| Sharpness | Acuity 43.7 cycles per degree median of 1 behavioural rows (method priority rule) | Measured | [3] |
| Field of view | Binocular overlap 47° median of 1 rows (eyes-at-rest rows preferred) | Measured | [4] |
| Total field of view 277° rule: total = 360 - blind area | Derived | [4] | |
| Blind area behind the head 83° | Measured | [4] | |
| Eye placement lateral frontal if binocular overlap >= 60 deg, else lateral | Derived | [4] | |
| Sharp zones (foveas) | Number of foveas 2 retinal topography | Measured (not re-verified) | [5] |
| Fovea type deep central + shallow temporal | Measured (not re-verified) | [5] | |
| Night vision | Activity pattern diurnal mode of 5 rows (of 5 rows): diurnal; not_nocturnal; photopic | Measured (not re-verified) | [6][7][8][9][10] |
| Rods vs cones cone-dominated nocturnal -> rod-dominated; crepuscular / cathemeral / mixed -> mixed; diurnal -> cone-dominated | Derived | [6][7][8][9][10] | |
| Motion (flicker fusion) | Flicker fusion frequency 77.7 Hz median of 1 bright-light rows (behavioural/whole-eye ERG rows; all rows: [77.7]) | Measured | [11] |
Related animals
- Black kite same vision type
- Egyptian vulture same vision type
- Griffon vulture same vision type
- Red-tailed hawk same vision type
- Turkey vulture same vision type
- Bald eagle same vision type
More birds: all birds with measured vision data.
Sources
- Lind O, Mitkus M, Olsson P, Kelber A. 2014. Ultraviolet vision in birds: the importance of transparent eye media. Proc R Soc B 281:20132209. Table 1. doi.org/10.1098/rspb.2013.2209
- Longcore T. 2023. A compendium of photopigment peak sensitivities and visual spectral response curves of terrestrial wildlife to guide design of outdoor nighttime lighting. Basic Appl Ecol 73:40-50. doi:10.1016/j.baae.2023.09.002. doi.org/10.5281/zenodo.8432720
- Caves EM, Brandley NC, Johnsen S (2018) Visual acuity and the evolution of signals. Trends Ecol Evol 33:358-372. Supplementary Tables S1-S3.. doi.org/10.1016/j.tree.2018.03.001
- Tyrrell LP, Moore BA, Loftis C, Fernandez-Juricic E 2017 (data 2017). The hawk-eyed songbird: retinal morphology, eye shape, and visual fields of an aerial insectivore. Am Nat 189(6). Dryad doi:10.5061/dryad.n7140.. doi.org/10.1086/691404
- Potier S, Mitkus M, Bonadonna F, Duriez O, Isard P-F, Dulaurent T, Mentek M, Kelber A 2017. Eye size, fovea, and foraging ecology in accipitriform raptors. Brain Behav Evol 90: 232-242. Supplementary material (Tables S1, S2).. doi.org/10.1159/000479783
- Light conditions and the evolution of the visual system in birds (figshare dataset, SupplementaryDataset1). doi.org/10.6084/m9.figshare.22116371.v3
- Choiniere JN, Neenan JM, Schmitz L, Ford DP, Chapelle KEJ, Balanoff AM, Sipla JS, Georgi JA, Walsh SA, Norell MA, Xu X, Clark JM, Benson RBJ. 2021. Evolution of vision and hearing modalities in theropod dinosaurs. Science 372:610-613. doi:10.1126/science.abe7941. Data: https://osf.io/teq73/. doi.org/10.1126/science.abe7941
- Wilman H, Belmaker J, Simpson J, de la Rosa C, Rivadeneira MM, Jetz W. 2014. EltonTraits 1.0: species-level foraging attributes of the world's birds and mammals. Ecology 95:2027. BirdFuncDat.txt. doi.org/10.6084/m9.figshare.3559887.v1
- Schmitz L, Motani R. 2011. Science 332:705-708, SOM. doi.org/10.1126/science.1200043
- Moura et al. 2024. A phylogeny-informed characterisation of global tetrapod traits addresses data gaps and biases. PLoS Biol 22:e3002658. TetrapodTraits v3.0.1.. doi.org/10.5281/zenodo.22536349
- Lafitte A, Sordello R, Legrand M, Nicolas V, Obein G, Reyjol Y. 2022. A flashing light may not be that flashy: A systematic review on critical fusion frequencies. PLoS ONE 17(12): e0279718. S10 File (CFF database). doi.org/10.1371/journal.pone.0279718
- Healy K, McNally L, Ruxton GD, Cooper N, Jackson AL. 2013. Metabolic rate and body size are linked with perception of temporal information. Animal Behaviour 86:685-696. Table 1. doi.org/10.1016/j.anbehav.2013.06.018
- Inger R, Bennie J, Davies TW, Gaston KJ. 2014. Potential biological and ecological effects of flickering artificial light. PLoS ONE 9(5): e98631. Table 3. doi.org/10.1371/journal.pone.0098631
Every value cites its sources (all sources). Data: catalogue-v1, built 2026-09-29. Accuracy notes: how accurate is this?